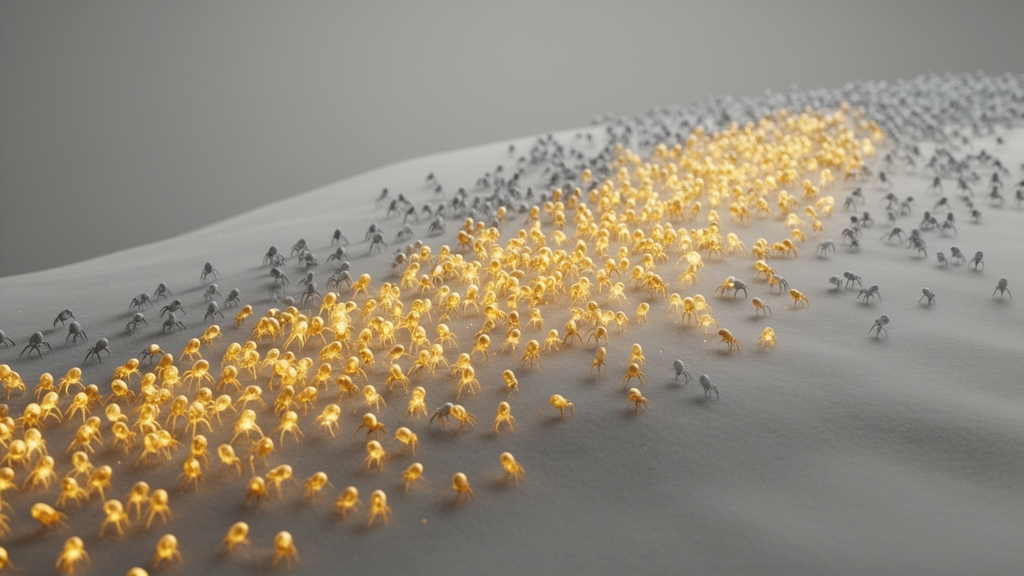
Every birth in a population comes with a death. In the classic mathematical description of evolution known as the Moran process, one individual is chosen to reproduce and another is chosen to die, and if both happen to be the same type of individual, the reproductive event changes nothing. Now a team of theoretical researchers has quantified just how much an evolving lineage can gain by eliminating that waste. In a study published in PLOS Computational Biology, Michal Pecho, Josef Tkadlec and Martin A. Nowak introduce a phenotype they call a replacer: an individual whose offspring, whenever possible, specifically displaces a member of the other type rather than a random neighbor. The result is a striking set of mathematical theorems showing that replacers enjoy a dramatically higher chance of taking over a population and, once established, are extraordinarily hard to dislodge.
The standard Moran process unfolds in discrete steps in a population of N individuals. Each individual carries a reproductive rate, and the probability of being selected as a parent is proportional to that rate. The parent then produces an offspring that replaces another individual, chosen uniformly at random. When the reproducing and dying individuals share a type, the population composition is unchanged and the step is, in effect, wasted. A replacer avoids this entirely: when selected for reproduction, its offspring replaces a random individual among those of a different type, provided such an individual exists. The authors contrast replacers with what they call oblivious mutants, the standard individuals that displace targets at random without regard to type.
To measure the success of this competitive strategy, the researchers calculated three quantities: the fixation probability, meaning the chance that a single invading mutant eventually converts the whole population; the elimination probability, the chance that an established mutant population is wiped out by a single resident invader; and the expected abundance of mutants at a mutation-selection equilibrium, where every birth carries a small probability of mutation to the opposite type. They analyzed these quantities for well-mixed populations, in which any individual can replace any other, and for a one-dimensional lattice with periodic boundary conditions, arranged as a cycle in which offspring migrate only to neighboring sites.
The fixation results reveal a sharp asymmetry. For a single neutral replacer, one whose reproductive rate equals that of the residents, the fixation probability in a well-mixed population of size N is proportional to a quantity that, while still tending to zero as N grows, decreases far more slowly than the standard 1/N fixation probability of an oblivious neutral mutant. The advantage only appears once the replacer lineage grows: the authors show that with a single mutant, being a replacer confers no benefit at all, but as the number of replacers increases, the forward bias of the population, the ratio of the probability that the mutant count rises to the probability that it falls, grows with the mutant frequency. For non-neutral mutants the fixation picture changes less. A deleterious replacer still has an exponentially small fixation probability in a large population, and an advantageous replacer tends to the same positive fixation constant as an advantageous oblivious mutant.
The defensive side of the story is where replacers truly excel. For oblivious mutants, the elimination probability of an established population facing a single resident is again 1/N in the neutral case, and for deleterious mutants it tends to a positive constant, meaning established disadvantageous lineages remain highly vulnerable to invasion. For replacers, by contrast, the elimination probability is exponentially small in the population size, regardless of whether the mutant is beneficial or deleterious. Once replacers become established, they are therefore extremely unlikely to be wiped out, even when their reproductive rate is reduced. In the authors’ framing, replacers enjoy strong evolutionary stability that oblivious types lack.
That stability translates into dominance at equilibrium. In the mutation-selection process, where each reproductive event has a probability u of producing an offspring of the opposite type, the researchers tracked the long-term average abundance of mutants. Replacers form a majority of the population even at reproductive rates below parity, where oblivious mutants with the same rate would remain a minority. In the limit of low mutation rate, the population composition is governed by the ratio of fixation to elimination probability, and the authors identify a threshold reproductive rate below which even replacer status cannot compensate for the disadvantage. Curiously, for large population sizes and small mutation rates, that threshold implies that a successful replacer can reproduce at a relative rate as low as 1/e, roughly 0.37, and still dominate the equilibrium.
The researchers also asked how much reproductive rate an individual could afford to sacrifice in exchange for the replacer phenotype and still match the performance of a neutral oblivious mutant. The answer depends on the measure of success and the population size. To match fixation probability, the tolerable cost peaks at populations of size eight, where it exceeds 0.27, and remains above 0.16 at a population size of 100, before tending to zero for very large populations. To match elimination probability, the cost approaches its theoretical maximum: even extremely disadvantageous replacers match the elimination probability of neutral non-replacers. At the mutation-selection equilibrium with low mutation rates, the same near-maximal cost applies.
Spatial structure amplifies these effects. On a cycle, where oblivious mutants fare exactly as they do in a well-mixed population, replacers behave differently in ways the authors compute exactly. For a replacer with reproductive rate below one half, becoming a replacer effectively doubles the mutant’s reproductive rate; for rates above one half, it contributes an additive boost of one half. Most strikingly, the fixation probability of a single neutral replacer invading a large cyclically structured population approaches the constant 1/3, rather than vanishing with population size, and on the cycle replacers dominate the mutation-selection equilibrium at low mutation rates whenever their relative reproductive rate exceeds one half, even at rates as low as 0.5.
Although the model is primarily a mathematical construction, the authors point to natural settings where replacer-like behavior appears. During cancer evolution in the fruit fly Drosophila, the dMyc transcription factor transforms cells into super-competitors that actively trigger apoptosis in adjacent cells that are not super-competitors themselves, so those cells behave like replacers. In fungal competition, hyphae can direct antagonistic growth preferentially toward genetically distinct neighbors, inhibiting, killing or overgrowing them through hyphal interference and necrotrophic mycoparasitism. And in cultural evolution, humans spreading opinions tend to concentrate persuasion on contacts who hold the opposing view rather than preaching to the choir.
The authors also show that the dynamics of neutral replacers versus oblivious individuals closely mirrors an evolutionary game: in a well-mixed population, the fixation probabilities of the two types match those of a game in which replacers receive payoff from one another while oblivious individuals do not, and a similar correspondence holds on cycles. For general graphs, however, no simple payoff matrix captures the dynamics, since tracking the exact configuration of the population becomes necessary. The study is limited to two population structures, the well-mixed population and the one-dimensional cycle, and the authors flag several open directions, including partial replacers that express the phenotype only with some probability, and smarter replacers that choose the most advantageous replacement targets. The core message, however, stands on its own: in these models, competitive efficiency can outweigh raw reproductive speed, allowing a slower-breeding lineage to dominate a population simply by never wasting a birth.
Subject of Research: Mathematical analysis of a replacer phenotype in stochastic evolutionary dynamics
Article Title: The evolutionary advantage of replacers in the Moran process
Article References: Pecho, M., Tkadlec, J., & Nowak, M. A. (2026). The evolutionary advantage of replacers in the Moran process. PLOS Computational Biology, 22(10), e1014892. https://doi.org/10.1371/journal.pcbi.1014892
Image Credits: AI Generated
DOI: 10.1371/journal.pcbi.1014892
Keywords: evolutionary dynamics, Moran process, fixation probability, mutation-selection equilibrium, replacer phenotype, evolutionary game theory, population genetics, spatial structure, elimination probability, theoretical biology, evolutionary, advantage
Cite Scienmag News
Gavin Prescott. (October 29, 2026). Wasted Births, Big Wins: New Model Shows How ‘Replacer’ Traits Dominate Evolution. Scienmag. https://scienmag.com/wasted-births-big-wins-new-model-shows-how-replacer-traits-dominate-evolution/
Gavin Prescott. "Wasted Births, Big Wins: New Model Shows How ‘Replacer’ Traits Dominate Evolution." Scienmag, 29 October 2026, https://scienmag.com/wasted-births-big-wins-new-model-shows-how-replacer-traits-dominate-evolution/. Accessed 29 October 2026.
Gavin Prescott. "Wasted Births, Big Wins: New Model Shows How ‘Replacer’ Traits Dominate Evolution." Scienmag. October 29, 2026. https://scienmag.com/wasted-births-big-wins-new-model-shows-how-replacer-traits-dominate-evolution/