

Tidal marshes are among the planet’s most celebrated carbon vaults. Their waterlogged sediments trap sediment, nurture lush plant growth, and slow the microbes that would otherwise exhale buried carbon back into the atmosphere. But a new study suggests that the mathematical machinery scientists use to estimate how much carbon dioxide these soils release may contain a subtle yet consequential flaw, one rooted in a phenomenon invisible to the naked eye: the patchy, millimetre-scale geography of oxygen around plant roots.
The research, published in the journal Biogeosciences by Youssef Saadaoui of the Helmholtz-Zentrum Hereon and colleagues at the University of Hamburg and partner institutions, set out to quantify what mathematicians call aggregation bias in marsh carbon flux estimates. The team’s central finding is striking in its simplicity. When models collapse the wildly variable oxygen conditions of the marsh rhizosphere into a single average value, they overestimate microbial carbon dioxide production by roughly 12 percent on average. Because the amount of carbon a marsh stores is essentially the difference between what plants put into the soil and what microbes breathe out, a systematic overestimate of respiration translates directly into an underestimate of the marsh carbon sink.
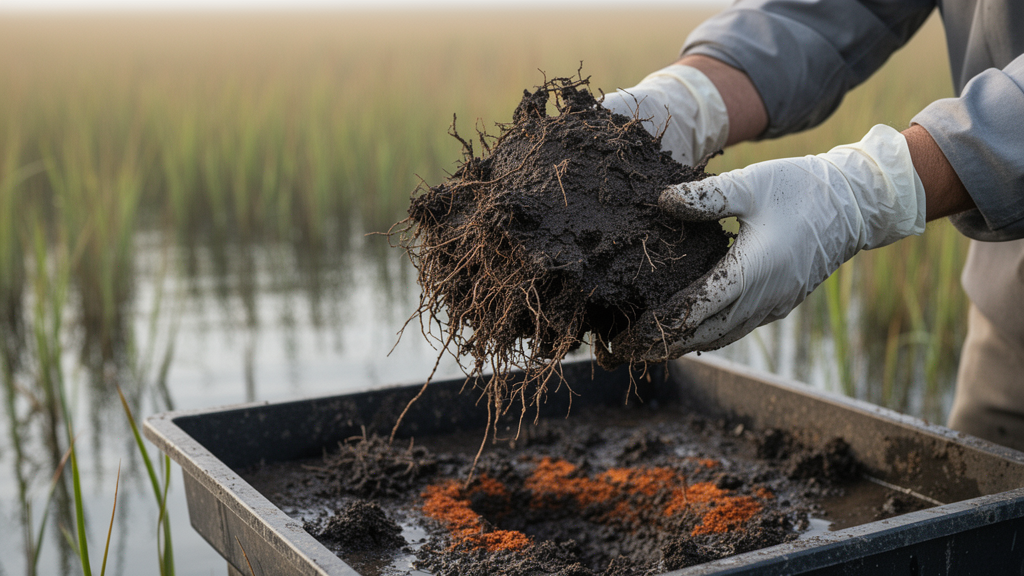
To understand why this happens, it helps to picture the underground world of a salt marsh. Oxygen in these soils is anything but uniform. Marsh grasses such as Spartina pipe air down through internal channels in their roots, releasing it into the surrounding sediment through a process known as radial oxygen loss. This creates tiny oxic halos around root surfaces. Just millimetres away, however, oxygen plunges to nearly zero, consumed by microbes and by the chemical re-oxidation of reduced compounds such as dissolved sulfide, iron sulfides, and ammonium. Tides, drainage, sediment texture, and plant physiology all churn this mosaic, so that within a few centimetres a microbe might inhabit anything from a well-aerated hotspot to an effectively airless pocket.
Most ecosystem and land-surface models, however, do not see this patchwork. They represent belowground redox conditions with a single bulk value, an average oxygen level or a uniform moisture scalar applied across an entire grid cell or plant type. The trouble is that microbial respiration does not respond linearly to oxygen. Instead, it follows a saturating, Michaelis-Menten-type curve: when oxygen is scarce, a little more of it produces a large boost in decomposition, but once oxygen is plentiful, additional amounts barely matter. When a curved response like this is evaluated at an average input rather than averaged across the full range of inputs, the result diverges from reality, a classic consequence of Jensen’s inequality, a mathematical principle familiar to ecologists since the early 1990s.
Saadaoui and colleagues turned this abstract principle into a concrete number for marsh soils. They calibrated a widely used enzyme-kinetic respiration model, the Dual Arrhenius and Michaelis-Menten framework, against long-term laboratory incubations of marsh soils collected from the Elbe estuary in Germany. In those incubations, soils of varying organic carbon content were held at controlled temperature and moisture for up to 465 days while carbon dioxide production was tracked by gas chromatography. Crucially, the incubations served only to pin down the carbon-side kinetics of the model; oxygen effects were then manipulated separately in the aggregation experiments, with temperature and substrate availability held fixed so that any difference between model configurations could be attributed purely to how oxygen was treated.
The team then ran the same calibrated model in two configurations. In the uniform configuration, respiration was evaluated at the arithmetic mean of a prescribed rhizosphere oxygen distribution, generated from realistic variation in water content and air-filled porosity driven by tidal flooding and drainage. In the heterogeneous configuration, respiration was averaged across the full oxygen distribution, capturing the fact that some microbes live in oxygen-rich zones while others barely receive any. For the gas-phase oxygen proxy, the uniform approach produced fluxes consistently higher than the heterogeneous average, with a mean bias of about minus 12 percent, meaning the single-average treatment overestimated aerobic carbon dioxide release by roughly a tenth. The overestimate ranged between about 6 and 13 percent depending on the microbial oxygen affinity assumed.
The study also revealed when the bias matters and when it does not. The key quantity is the ratio of mean oxygen concentration to the half-saturation constant, the oxygen level at which microbes achieve half their maximum respiration rate. When mean oxygen sits far below this threshold, the respiration response is nearly linear and averaging errors vanish; the dissolved-phase oxygen proxy, whose concentrations are hundreds of times smaller than the gas-phase equivalent, produced a negligible bias of about 0.05 percent. When oxygen is effectively saturating, the response flattens and the bias again shrinks. The largest errors arise in the intermediate regime, where respiration is strongly limited by oxygen but not starved of it, and where spatial variability is substantial. Narrowing the oxygen distribution, as in a benchmark representing nearly saturated soils, reduced the bias to half a percent.
A diagnostic analysis confirmed the mechanism. By holding the mean oxygen constant and systematically increasing its variance with symmetric two-point mixtures, the researchers showed that the bias grows nearly linearly with variance, exactly as a second-order Taylor approximation based on the curvature of the oxygen-limitation term predicts. The bias remained negative across every distribution shape tested, including lognormal fields, indicating that the effect is a structural property of concave oxygen limitation rather than an artefact of any particular assumption. In practical terms, this means modellers can anticipate the error from just three pieces of information: the mean oxygen concentration, its variance, and a calibrated half-saturation constant.
The implications ripple outward to global carbon accounting. Published estimates place global salt-marsh carbon burial at roughly 10 to 21 teragrams of carbon per year, though the full range of published accumulation-rate estimates spans from about 0.9 to more than 31 teragrams. If a bias of around 12 percent were broadly representative of tidal marshes, correcting for it would raise inferred global sequestration by on the order of 1 to 2.5 teragrams of carbon per year, equivalent to roughly 0.1 to 0.25 gigatonnes over a century. The authors are careful to frame these as order-of-magnitude extrapolations rather than forecasts, and the corrected flux remains small beside fossil fuel emissions. Still, for blue carbon inventories and coastal greenhouse gas budgets, where marshes are counted among nature’s most efficient carbon sinks, a systematic error of this size is far from trivial.
The study also carries a broader lesson for Earth system science. As mechanistic, oxygen-explicit respiration schemes migrate into regional and global models, the way oxygen is aggregated within each coarse grid cell becomes a first-order control on predicted fluxes, not a secondary detail. The researchers offer modellers a lightweight remedy: a curvature-based correction factor derived from the local oxygen variance, which their tests show can remove most of the bias when variability is modest. Where variability is large or poorly constrained, propagating a plausible range of oxygen variance into flux uncertainty is the more honest option. They further caution that defining the uniform baseline in terms of mean water content rather than mean oxygen can, in extreme cases, even flip the apparent sign of the effect. Realising the full promise of these diagnostics, the authors note, will require more high-resolution microelectrode and planar optode measurements of rhizosphere oxygen across tidal elevations, plant species, and seasons, along with better constraints on microbial oxygen kinetics in marsh soils. For now, the message is clear: beneath the quiet surface of a marsh, the invisible architecture of oxygen is quietly reshaping how much carbon we think these ecosystems can hold.
Subject of Research: Aggregation bias in modelled marsh soil carbon dioxide fluxes caused by millimetre-scale rhizosphere oxygen heterogeneity
Article Title: Quantifying aggregation bias in marsh carbon flux estimates caused by rhizosphere oxygen heterogeneity
Article References: Saadaoui, Y., Beer, C., Mueller, P., Neiske, F., Becker, J. N., Eschenbach, A., & Porada, P. (2026). Quantifying aggregation bias in marsh carbon flux estimates caused by rhizosphere oxygen heterogeneity. Biogeosciences, 23(19), 6803-6816. https://doi.org/10.5194/bg-23-6803-2026
Image Credits: AI Generated
Keywords: tidal marshes, blue carbon, rhizosphere oxygen, heterotrophic respiration, aggregation bias, Jensen's inequality, Michaelis-Menten kinetics, DAMM model, carbon flux, soil incubation, Elbe estuary, biogeochemical modelling
Cite Scienmag News
Violet Maxwell. (October 9, 2026). Hidden Oxygen Mosaics in Marsh Soils Skew Carbon Models by 12 Percent. Scienmag. https://scienmag.com/hidden-oxygen-mosaics-in-marsh-soils-skew-carbon-models-by-12-percent/
Violet Maxwell. "Hidden Oxygen Mosaics in Marsh Soils Skew Carbon Models by 12 Percent." Scienmag, 9 October 2026, https://scienmag.com/hidden-oxygen-mosaics-in-marsh-soils-skew-carbon-models-by-12-percent/. Accessed 9 October 2026.
Violet Maxwell. "Hidden Oxygen Mosaics in Marsh Soils Skew Carbon Models by 12 Percent." Scienmag. October 9, 2026. https://scienmag.com/hidden-oxygen-mosaics-in-marsh-soils-skew-carbon-models-by-12-percent/


