Salmonella enterica remains one of the most consequential bacterial pathogens of humans, with estimates ranging from 200 million to one billion infections each year, spanning self-limiting gastroenteritis to life-threatening typhoid fever. The 2024 WHO Bacterial Priority Pathogens List ranks fluoroquinolone-resistant Salmonella Typhi among the highest-priority community-acquired pathogens, and resistance is rising. Against this backdrop, a new open-access review in Discover Bacteria by Ronan C. Jensen and Gregory D. Fairn argues that a single injected bacterial protein deserves renewed attention: SopB, also known as SigD, an effector the authors describe as contributing to virtually every stage of infection, from the first moments of cell entry to the establishment of the intracellular replicative niche.
SopB was first identified in the 1990s as a secreted protein required for fluid accumulation and neutrophil influx in the bovine ligated ileal loop model, and independently recovered in a screen for genes driving epithelial cell invasion. The unifying biochemical insight came when researchers showed that recombinant SopB possesses inositol polyphosphate 4-phosphatase activity, hydrolysing both soluble inositol phosphates and the lipid PtdIns(3,4,5)P3 in vitro. This was the first demonstration of phosphoinositide phosphatase activity in any bacterial type III secretion system effector, and it founded a family that now includes IpgD from Shigella and VPA0450 from Vibrio parahaemolyticus. The protein is a 561-residue polypeptide of roughly 62 kilodaltons, built from a C-terminal catalytic region carrying the conserved Cys-X5-Arg motif, and an N-terminal module that binds the host GTPase Cdc42.
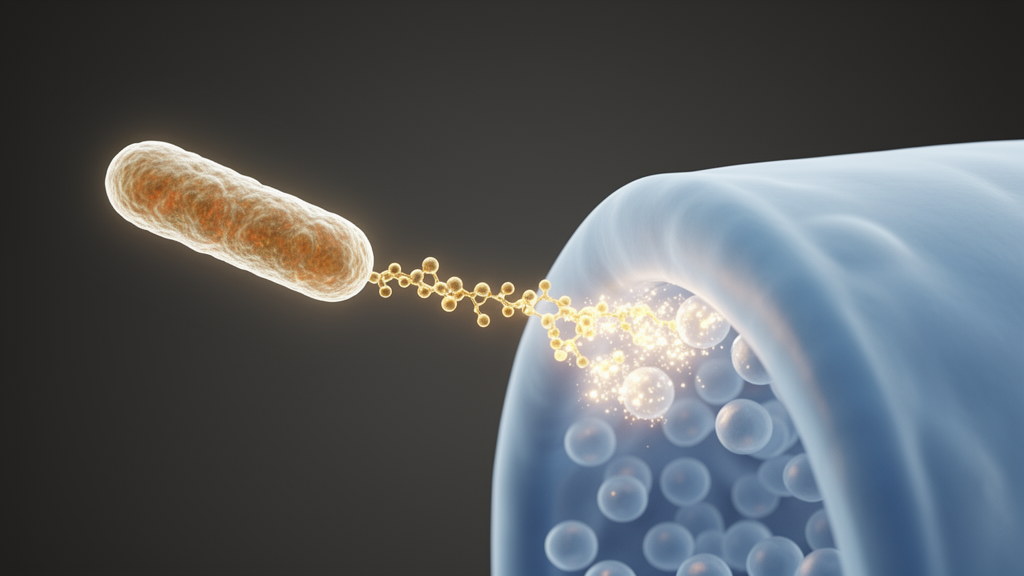
The most consequential recent discovery, and the centrepiece of the review, is that SopB is not merely a phosphatase. Walpole and colleagues demonstrated that SopB also possesses an intrinsic phosphotransferase activity that operates independently of host PI 3-kinases and of ATP. During the catalytic cycle, a covalent cysteinyl-phosphate intermediate forms at Cys460. Instead of always being resolved by water, as in a canonical phosphatase reaction, that phosphate can be attacked by the 3-hydroxyl of another phosphoinositide headgroup, transferring the phosphate to the 3-position. The result is the direct generation of PtdIns(3,4)P2, and transiently PtdIns(3,4,5)P3, from PtdIns(4,5)P2. The reaction was reconstituted with recombinant SopB acting on chemically defined liposomes in a cell-free system devoid of ATP, divalent cations and any host enzymes, and was further validated by expressing SopB in budding yeast, an organism that lacks all class I and class II PI 3-kinases yet still produced PtdIns(3,4)P2 upon SopB induction. The same activity was demonstrated for IpgD, indicating that the capability is ancestral to this effector family.
This finding reframes more than two decades of literature. SopB has long been known as a potent activator of the pro-survival kinase Akt in epithelial cells, with the response both dependent on its catalytic activity and persisting for many hours after invasion. The prevailing model held that SopB indirectly elevated the Akt-activating lipids by engaging host phosphoinositide 3-kinases, and several lines of evidence did support a host-kinase contribution: pharmacological PI3K inhibition partially reduced Akt activation, PTEN overexpression abolished it, and an unbiased screen identified more than 50 host kinases whose depletion dampened Akt phosphorylation during invasion. But no single host kinase fully accounted for the response. The review argues that the gap is now closed: the relevant Akt-activating lipid is generated by SopB itself, and the earlier observations of partial PI3K dependence are best understood as auxiliary inputs layered on top of the effector’s own synthesis.
Time-resolved HPLC-MS analysis reveals that the two enzymatic activities are not alternative modes but sequential phases of a single reaction trajectory. Acting on PtdIns(4,5)P2-containing liposomes, SopB first generates a transient pulse of 3-phosphorylated, pro-survival and pro-invasion lipids, which are then progressively dephosphorylated, ultimately leaving phosphatidylinositol as the dominant product. During actual infection, roughly half of the cellular pool of PtdIns(4,5)P2 is metabolized during invasion. The biological consequence is a kinetically structured output: a brief burst of 3-phosphorylated lipids during host cell engagement, followed by sustained depletion of negatively charged phosphoinositides as the Salmonella-containing vacuole matures and its surface charge dissipates. Accessory residues including Lys525 and Lys528 selectively affect phosphotransferase output, providing genetic tools to dissect the two activities independently, something the conserved Cys-X5-Arg motif alone never allowed.
The cytoprotective consequences are substantial. Knodler and colleagues showed that SopB is required to suppress caspase-3 cleavage in infected epithelial cells and confers resistance to camptothecin-induced apoptosis, both phenotypes dependent on continuous Akt signalling. Protection extends to B lymphocytes, where SopB-driven Akt activation phosphorylates the Hippo pathway effector YAP, preventing its nuclear translocation and thereby suppressing NLRC4 inflammasome assembly and IL-1β release. In epithelial cells, an additional layer of protection arises from SopB binding and sequestering the host E3 ligase TRAF6, preventing its mitochondrial recruitment and attenuating ROS-driven apoptosis through a mechanism at least partially independent of Akt. The review frames this strategically: premature apoptosis would expose the bacteria to extracellular immune effectors and terminate intracellular replication, so sustaining Akt activation extends the lifespan of the infected cell long enough to support multiple rounds of bacterial replication.
Remarkably, that window of protection is extended by a second, distinct wave of type III secretion system 1 effector translocation. Finn and colleagues showed that intracellular Salmonella that have entered the host cell cytosol deliver SopB and SipA into hyper-replicative, bacteria-containing cells well after the initial invasion-phase translocation is complete, reactivating Akt and prolonging cell survival. This late translocation is translocon-independent, unlike the canonical pore-forming mechanism used during invasion, revealing the secretion system as temporally bipartite. SopB’s unusual longevity makes such late action possible: whereas most SPI-1 effectors are rapidly turned over, SopB remains detectable for up to 12 hours post-invasion, bridging the temporally distinct activities of the two secretion systems and conditioning the vacuole for the later SPI-2 effector network.
SopB also acts through entirely non-enzymatic means. In U2OS cells, Zhao and colleagues showed that its N-terminal Cdc42-binding domain engages and activates Cdc42, driving MEK1/2-dependent assembly of a vimentin cage around the maturing vacuole that supports vacuolar integrity and bacterial replication. The authors of the review flag two caveats: the evidence derives largely from a single study in an osteosarcoma cell line not widely used in the field, so confirmation in enterocytes and macrophages is needed, and the extent to which SopB directly activates Cdc42, rather than merely binding it, has been debated. Structurally, the N-terminal domain mimics a host guanine nucleotide dissociation inhibitor, engaging the switch regions of Cdc42 and slowing nucleotide exchange. SopB also participates in a web of effector cooperation and antagonism: it cooperates with SopD, a Rab10 GTPase-activating protein, during membrane scission at the closing ruffle, while its phosphoinositide remodelling actively destabilizes the nascent vacuole, an effect counteracted by SopF, which preserves vacuole integrity and blocks ATG16L1 recruitment to suppress xenophagy.
Adding a further layer of regulation, SopB is itself a substrate of the host ubiquitin machinery. Mass spectrometry identified six lysine residues in its N-terminal region that are multiply mono-ubiquitinated after translocation, with TRAF6 and the E2 conjugating enzyme UbcH5c identified as the responsible enzymes. Crucially, this modification is regulatory rather than destructive: the intracellular half-life of SopB is unaffected by mutation of the ubiquitinated lysines. Two contemporaneous studies converged on a so-called ticket-to-ride model, in which ubiquitination redirects SopB from the plasma membrane to the vacuole and toggles its enzymatic output between the two compartments; a non-ubiquitinatable variant remains stranded at the plasma membrane and shows intensified, prolonged Akt activation. Jensen and Fairn propose a refinement, a ubiquitin-mediated electrostatic switch: ubiquitin conjugation neutralizes the positive charges by which SopB anchors to negatively charged membrane lipids, releasing it to relocate to Cdc42-enriched compartments. They outline testable predictions, including that charge-reducing substitutions should phenocopy ubiquitination.
The review closes with open questions and translational possibilities. A cryo-EM structure of SopB is now available in the Protein Data Bank, though the corresponding manuscript is still pending publication, and quantitative dissection of phosphatase versus phosphotransferase flux in living cells remains unresolved, as do SopB’s roles in macrophages, dendritic cells and primary enterocytes. The catalytic site offers a tractable target for anti-virulence inhibitors that would avoid the selective pressure driving antibiotic resistance, and SopB’s conservation across the roughly 16-effectors core shared by typhoidal and non-typhoidal serovars makes it a candidate antigen for next-generation vaccines. The authors also draw a direct line to oncology: epidemiological studies have linked chronic typhoid infection with gallbladder carcinoma, and repeated exposure to non-typhoidal Salmonella has been identified as an environmental risk factor for colon cancer, with effectors including SopB implicated through sustained Akt and MAPK activation. Direct generation of mitogenic phosphoinositides by a bacterial enzyme, they argue, offers a more parsimonious explanation than indirect modulation of host kinases, and positions SopB as a continuing discovery vehicle for otherwise inaccessible corners of cell biology.
Subject of Research: Multifunctional activities of the Salmonella effector protein SopB in manipulating host phosphoinositide signalling
Article Title: Enzymatic versatility of the salmonella effector SopB enables manipulation of host phosphoinositide signalling
Article References: Jensen, R. C., & Fairn, G. D. (2026). Enzymatic versatility of the salmonella effector SopB enables manipulation of host phosphoinositide signalling. Discover Bacteria, 3(1), Article 19. https://doi.org/10.1007/s44351-026-00056-8
Image Credits: AI Generated
DOI: 10.1007/s44351-026-00056-8
Keywords: Salmonella enterica, SopB, type III secretion system, phosphoinositides, phosphotransferase, Akt signalling, Salmonella-containing vacuole, vimentin, ubiquitination, Cdc42, bacterial effector, host-pathogen interaction
Cite Scienmag News
Kristina Jarvis. (October 28, 2026). Salmonella’s SopB protein makes a key signalling lipid without host kinases. Scienmag. https://scienmag.com/salmonellas-sopb-protein-makes-a-key-signalling-lipid-without-host-kinases/
Kristina Jarvis. "Salmonella’s SopB protein makes a key signalling lipid without host kinases." Scienmag, 28 October 2026, https://scienmag.com/salmonellas-sopb-protein-makes-a-key-signalling-lipid-without-host-kinases/. Accessed 28 October 2026.
Kristina Jarvis. "Salmonella’s SopB protein makes a key signalling lipid without host kinases." Scienmag. October 28, 2026. https://scienmag.com/salmonellas-sopb-protein-makes-a-key-signalling-lipid-without-host-kinases/