

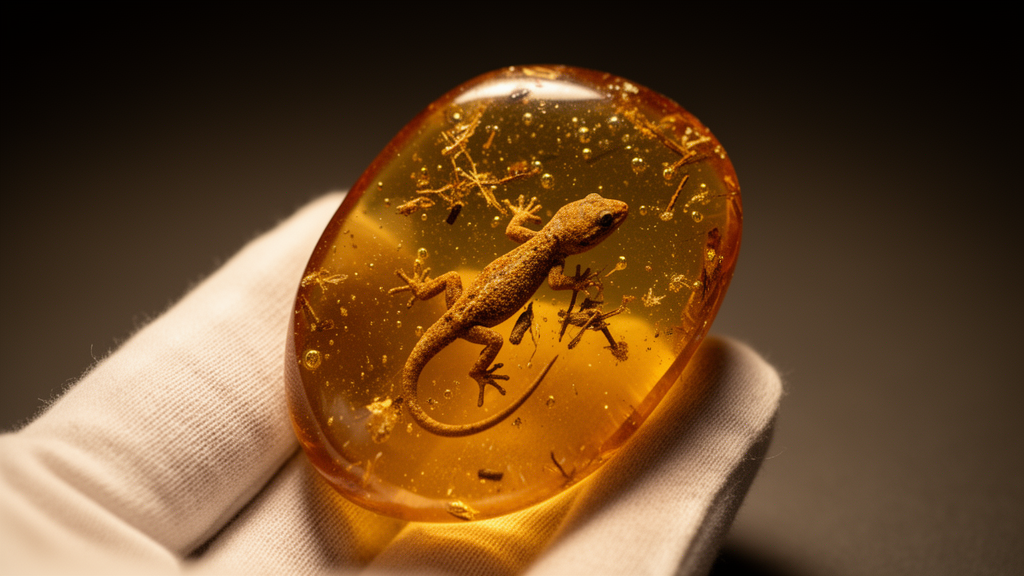
A pair of tiny lizards trapped in Burmese amber roughly 99 million years ago has yielded one of the rarest prizes in vertebrate palaeontology: direct evidence of male genital anatomy in a fossil squamate. The two specimens, described in the Swiss Journal of Palaeontology as a new genus and species, Carinasquama rusmithii, preserve almost the entire scaled skin of the animals even though their skeletons are largely gone. In one of them, a swelling at the base of the tail matches the hemipenal bulge seen in living male lizards, marking the animal as male and documenting the presence of paired copulatory organs, or hemipenes, in gecko relatives during the mid-Cretaceous.
Sexing fossils is notoriously difficult. Palaeontologists usually work from skeletal features, but isolated bones rarely carry reliable clues. In some assemblages, sexual dimorphism can be detected through differences in ornamentation or through multivariate analyses of shape. Mammals often show size differences and specialised armaments such as tusks, antlers and horns, and their genitalia include the bony baculum, which varies remarkably between species. Among non-avian dinosaurs, dimorphism has proved elusive, although plate morphology in some Stegosaurus species has been interpreted as evidence of two forms, and anatomical differences in pterosaurs remain among the most compelling cases of sexual dimorphism in fossil reptiles.
Female sex can occasionally be inferred when embryos are preserved inside or beside a specimen, or when medullary bone is detected in sexually mature females, a tissue restricted to birds and some non-avian dinosaurs. The Mesozoic bird Confuciusornis sanctus, in which males bear two elongated ornamental tail feathers, has been sexed this way. But both embryos and medullary bone are temporary features, so they cannot diagnose the sex of an animal that is not gravid. In single fossil reptile specimens, especially males, osteological evidence of sex is usually absent, and many specimens remain unsexed.
Lizards offer some taxon-dependent clues. Males generally have larger heads, and some species show marked dimorphic traits such as the long snout of male Anolis brunneus or the head casque of the veiled chameleon. Among geckos, sexual size dimorphism is variable: a survey of 43 species found males larger in 13, females larger in 26, and the sexes equal in 4. Body size is therefore not generally reliable for estimating sex in fossil geckos, because there is no clear clade-wide trend and larger sample sizes would be needed. Additional structures associated with male geckos include post-cloacal bones, which have been tentatively identified in fossils as indications of male sex, although calcified hemibacula known from the genus Aristelliger have not yet been detected in any fossil lizard.
Soft tissues might display marked differences between sexes, including brightly coloured integument, integumentary ornaments such as horns or spurs, and enlarged femoral glands, precloacal organs or escutcheon scales, which are more developed in males although they may also be expressed in females. Reptiles have internal testes and retract the intromittent organ into the body cavity, so sex cannot be identified easily by viewing the animal externally. The male reproductive organs of squamates are paired hemipenes, a synapomorphy of the group whose development is attributed to the lack of expression of Sonic hedgehog signalling genes during embryological development. In many squamates, male sex may be determined by the presence of a hemipenal bulge located posteriorly to the cloaca, indicating that the hemipenes have been retracted into the base of the tail. While not apparent in all squamates, the bulge is seen in most male lizards and is absent in Sphenodon punctatus, the closest living relative of squamate reptiles.
The two new specimens were scanned using commercial micro-CT scanners at the University of Texas at Austin, the American Museum of Natural History and the University of Florida, and the reconstructed volume data were rendered and visualised using VGstudioMax. The holotype, housed in the National Museum of Scotland, measures approximately 16.24 millimetres snout-vent length, while the paratype, held at the Houston Museum of Natural Science, measures 21.92 millimetres. These sizes approximate the range of the smallest known extant geckos, including Sphaerodactylus ariasae and S. parthenophion at 16 to 18 millimetres. The body is depressed and the tail is as long as the body, covered by rings of juxtaposed oblong to pectinate scales that are multi-carinated with four to six parallel keels and surrounded by pigmented granules.
Only the paratype preserves portions of the skull, including a paired premaxilla, left maxilla, left dentary and part of the left coronoid. The premaxilla has seven tooth loci, the maxilla approximately 25, and the dentary about 24, with all teeth well spaced, isodont and mainly straight. The dentary is tubular with a fused Meckelian canal, and the putative splenial seems to have an anterolabial process and an anterolingual process, which supports the identification as a gekkotan. The holotype preserves a very complete appendicular skeleton, with humerus, radius, ulna, carpals and phalanges in the forelimbs and femur, tibia, fibula, tarsals and phalanges in the hind limbs. The distal epiphyses of the humeri and femora are unfused to the shafts, indicating that the individual is a juvenile, consistent with its smaller size compared to the paratype.
The integument is completely transparent, preserving the entire outline of the body. The head scales are small, homogeneous and granular, with no enlarged frontal or frontoparietal scales and no indication of eyelids, characters shared with extant gekkotans. In the holotype, scales near the cloaca preserve pigmentation compared to the surrounding body scales and clearly demarcate the opening of the cloaca. Posterior to the cloaca, near the base of the tail, there is a swelling interpreted as a hemipenal bulge, similar to that seen in many male lizards. The bulge is not evident in the paratype. Neither specimen shows femoral glands, precloacal organs or escutcheon scales, and none has adhesive subdigital pads, suggesting a more terrestrial than scansorial habit that contrasts with other geckos in Burmese amber.
The phylogenetic placement of Carinasquama rusmithii is uncertain, but it shares many derived characters with geckos and is provisionally placed in the total group Pan-Gekkota. Among living gekkotans, it has been estimated that the ancestor lacked toe pads and that these structures originated multiple times with several subsequent reversals, although later works have argued that exclusion of detailed morphological evidence contributed to the idea of a single origin. Burmese amber fossils document both padless and pad-bearing gekkotans during the mid-Cretaceous, indicating that ground-dwelling and scansoriality were already present at a time estimated for the origin of the crown clade of geckos. Earlier Jurassic pan-gekkotans such as Eichstaettisaurus, Ardeosaurus and Limnoscansor lack evidence of toe pads but show adaptations to climbing, including a symmetrical foot and elongated penultimate phalanges.
Evidence of hemipenal structures seen here, together with cloacal bones described in Lower Cretaceous lizards, hints at the early evolution of the hemipenes. Total group Squamata likely evolved in the Late Permian or Early Triassic and diversified greatly by the mid-Cretaceous, with many lizards from this time being either stem-squamates or basal members of extant clades. Today, squamates exhibit an extreme morphological variety of hemipenes, and this could have been an additional factor associated with their increased diversification and speciation during the Cretaceous. The ancestral state of the amniote penis was likely a single mid-line phallus, which is lost along the lepidosaurian lineage, with squamates possessing paired hemipenes and Sphenodon lacking a phallus. Three hypotheses exist on the ancestral lepidosaurian state: a single phallus that diverged as the lineages split, a paired hemipenis eventually lost in rhynchocephalians, or a phallus lost in lepidosaurs and re-evolved in squamates. The authors call for future work to pay close attention to mineralised genital structures like postcloacal bones and penal spines, and to evidence of soft tissues associated with sex in exceptionally preserved fossil specimens. The specimens were sourced following the recommendations of the Myanmar working group of the Society of Vertebrate Paleontology, and the holotype was donated to the National Museum of Scotland by Dr. Ru D. A. Smith, whose generosity the authors hope might inspire other collectors to make such controversial fossils more accessible for future studies.
Subject of Research: Male hemipenal anatomy preserved in mid-Cretaceous Burmese amber geckos
Article Title: Evidence of male anatomy in a mid-Cretaceous Burmese miniaturised amber gecko
Article References: Evidence of male anatomy in a mid-Cretaceous Burmese miniaturised amber gecko. (n.d.). https://doi.org/10.3897/sjp.145.188227
Image Credits: AI Generated
Keywords: amber fossils, geckos, hemipenes, Cretaceous, Myanmar, palaeontology, sexual dimorphism, micro-CT, Squamata, Carinasquama rusmithii, Evidence, male
Cite Scienmag News
Gavin Prescott. (October 16, 2026). Evidence of male anatomy in a mid-Cretaceous Burmese miniaturised amber gecko. Scienmag. https://scienmag.com/evidence-of-male-anatomy-in-a-mid-cretaceous-burmese-miniaturised-amber-gecko/
Gavin Prescott. "Evidence of male anatomy in a mid-Cretaceous Burmese miniaturised amber gecko." Scienmag, 16 October 2026, https://scienmag.com/evidence-of-male-anatomy-in-a-mid-cretaceous-burmese-miniaturised-amber-gecko/. Accessed 16 October 2026.
Gavin Prescott. "Evidence of male anatomy in a mid-Cretaceous Burmese miniaturised amber gecko." Scienmag. October 16, 2026. https://scienmag.com/evidence-of-male-anatomy-in-a-mid-cretaceous-burmese-miniaturised-amber-gecko/


